
Biophysics of Leaf Energy Balance and Leaf–Air Coupling Mechanics
The thermal state of a plant leaf is governed by fundamental biophysical principles that regulate heat dissipation and water loss under fluctuating environmental conditions. Leaf temperature represents the precise point of equilibrium in the leaf energy budget, balancing incoming radiation against thermal loss mechanisms. Analyzing these energy fluxes provides critical insight into the microclimatic conditions that surround plant foliage. Under conditions where thermal dissipation is inadequate, extreme heat stress can cause irreparable cellular damage and inhibit photosynthetic efficiency.
The total radiative forcing incident on a leaf varies significantly depending on solar position and atmospheric coverage. Typical environmental scenarios include clear skies at midday (approximately 1400 W m⁻²), cloudy conditions at midday (1100 W m⁻²), and low-angle radiation during late afternoon under cloud cover (800 W m⁻²). If longwave radiation (thermal emission) serves as the sole pathway for dissipating absorbed energy, the resulting steady-state leaf temperatures can reach extreme levels.
Specifically, with an ambient air temperature of 35°C, relying exclusively on longwave radiation forces the leaf to reach lethal thermal thresholds: 62°C under high radiative forcing, 42°C under moderate forcing, and 18°C under low radiative forcing. Consequently, additional energy dissipation mechanisms—namely convective heat flux and latent heat release—are required to maintain physiological thermal stability.
Convective and Latent Heat Dissipation Mechanisms. Sensible heat flux describes heat transfer via convection driven by temperature gradients between the leaf surface and the surrounding air. Under calm atmospheric conditions with a minimal wind speed of 0.1 m s⁻¹, convective cooling reduces the leaf temperature by 14°C (down to 48°C) under high radiative forcing, and by 4°C (down to 38°C) under moderate forcing. As wind speed increases, convective heat exchange intensifies considerably. At 5 m s⁻¹, forced convection removes sensible heat at a rate that reduces leaf temperature from 62°C to 38°C under peak solar irradiance. Conversely, when leaves experience low radiative forcing, convection can warm the leaf tissue, transferring thermal energy from the warmer surrounding air to the cooler leaf.
Latent heat flux, mediated by transpiration (evaporative water loss through stomatal pores), acts as a highly efficient cooling mechanism. Under calm conditions (0.1 m s⁻¹) and peak radiative forcing, transpirational cooling depresses leaf temperature by an additional 10°C, bringing it from 48°C down to 38°C.
When forced convection and transpiration act simultaneously at higher wind speeds (5 m s⁻¹), leaf temperature is successfully driven down from a critical threshold of 62°C to a physiologically stable 34°C.
This biophysical evaporative cooling process directly mirrors mammalian thermoregulation through perspiration. High relative humidity impairs the evaporative gradient, hindering cooling efficiency and heightening heat exposure, whereas low humidity facilitates rapid phase change and heat loss.
Theoretical Framework of Leaf–Air Coupling. The interaction between a leaf and its surrounding atmosphere is governed by a network of physical conductances that control energy and mass exchange. Sensible heat flux depends on boundary layer conductance, whereas latent heat flux is regulated by the combined action of boundary layer conductance and stomatal conductance operating in series.
To quantify these transport phenomena, Monteith (1965) along with Jarvis and McNaughton (1986) extended the classical Penman–Monteith equation to individual leaves. For a hypostomatous leaf (bearing stomata exclusively on the lower surface), assuming equivalent conductances for heat and water vapor transfer (g_bh = g_bw = g_b), the formulation is expressed as:
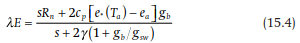
Where:
- λE represents the latent heat flux density (W m⁻²).
- s denotes the slope of the saturation vapor pressure curve relative to temperature (Pa K⁻¹).
- R_n is net radiation (W m⁻²).
- c_p is the volumetric heat capacity of air (J m⁻³ K⁻¹).
- e(T_a) - e_a* represents the atmospheric vapor pressure deficit (VPD).
- γ is the psychrometric constant (Pa K⁻¹).
- g_b is boundary layer conductance.
- g_sw is stomatal conductance to water vapor.
Stomatal Control and Limiting Coupling Regimes. The physiological impact of stomata on transpirational cooling varies between two extreme boundary conditions described by Jarvis and McNaughton (1986).
Decoupled Regime: Low Boundary Layer Conductance. When boundary layer conductance is extremely small, a stagnant, thick layer of still air develops around the leaf surface, effectively decoupling it from ambient atmospheric conditions. In this decoupled state, transpiration reaches the equilibrium evaporation rate:
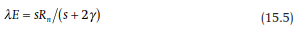
Under equilibrium conditions, transpirational flux becomes independent of stomatal conductance and is dictated almost entirely by the net radiation available to drive water vaporization.
Coupled Regime: High Boundary Layer Conductance. Conversely, when boundary layer conductance is exceptionally large, air movement strips away the stagnant boundary layer, establishing strong coupling between the leaf surface and the ambient atmosphere. Transpiration shifts to an imposed evaporation rate:
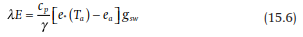
Under strong coupling, transpirational water loss is directly proportional to the ambient vapor pressure deficit and stomatal conductance. Any shift in stomatal opening causes an immediate, proportional change in transpiration rates.
Between these boundary conditions, leaves exhibit intermediate degrees of stomatal control. The precise degree of coupling is governed by leaf dimensions and localized wind speed. Small leaves possess high boundary layer conductance, leading to tight atmospheric coupling. Large leaves feature lower boundary layer conductance, maintaining a higher degree of decoupling. Moving air breaks down surface boundaries to promote strong coupling, whereas still air decouples the leaf microclimate from ambient atmospheric dynamics.
Date added: 2026-09-24; views: 3;